


 Spanish (pdf)
 Article in xml format
 Article references

 Automatic translation
 Send this article by e-mail
 Cited by SciELO
 Cited by Google
 Similars in
SciELO
 Similars in Google

 Permalink


INTRODUCTION
Pig farming represents an important economic and social production sector in several states of Brazil (Ramos et al., 2017), standing out as the fourth of the largest producers of meat exported worldwide. In addition, it is characterized as an animal production sector that employs small rural producers and encourages families to settle in the countryside and generate income (Ito et al., 2016).
The activity's growth has been a target of concern, especially regarding environmental issues, because when this production system is poorly designed or handled, enormous amounts of waste are generated and often launched into water bodies without previous treatment, which might pollute surface and underground waters (Velho et al., 2012). These wastes end up being carried by the water bodies and might directly interfere in biogeochemical cycles, as well as in the equilibrium of the biotic diversity and complexity of food webs (Margalef, 1983; Cunha and Calijuri, 2011).
In case aquatic ecosystems are enriched with nutrients - especially nitrogen and phosphorus compounds, a phenomenon called artificial eutrophication may occur, which harms the quality of water bodies and contributes for the increase of noxious microalgae (Anderson et al., 2002; Barreto et al., 2013). To obtain control of these compounds inside pig farms, it is necessary to optimize the recycling of organics and minimize effluent's leaching into soils and water bodies (Rigolot et al., 2010).
Phytoplankton microalgae are responsible for part of the primary production of an aquatic ecosystem, being paramount for its biological structure. These organisms contribute to the cycling of nutrients and its mineralization, as well as to the breakdown of organic matter, besides serving as the base of the food chain for several other organisms (Bichoff et al., 2016).
According to Margalef (1983), planktonic organisms function as "refined scanners of environmental conditions", thus reflecting in the dynamics ofthe ecosystem. In this sense, studies that include a taxonomic composition analysis and an evaluation of the phytoplankton community together with environmental variables are of great importance for monitoring water quality, assessing the health status of the environment, and inferring the probable causes of ecological damage (Gentil et al., 2008).
In addition to phytoplankton monitoring, other low-cost alternatives for the treatment of wastes derived from pig farming, which allow the reduction of potential environmental damages, are anaerobic digesters and lagoons of stabilization (Ramos et al., 2017). Phytoremediation is also a great alternative regarding the use of purifying agents, which is effective in reducing the negative effects of some effluents. This process uses aquatic plants such as macrophytes, which act by removing organic and inorganic pollutants (e.g., salts, metals, pesticides, and petroleum hydrocarbons), or by transforming there into less aggressive compounds (Pio et al., 2010; Pinaffi and Santos, 2019).
Immediate and corrective actions are needed for the improvement of effluent management in pig farms, such as the abovementioned ones, besides the implementation of efficient techniques for the treatment and correct discharge of manures, aiming to avoid both the quality and health loss of water bodies. According to Gliessman (2000), the adoption of production systems that maximize pasture use in pigs' feeding is highly needed, as it might reduce the use of synthetic inputs and improve the recycling of nutrients.
The main objective of this study was to evaluate the effects of pig farming effluent discharge, in the composition of phytoplankton assemblages and limnological variables in a lotic system.
MATERIAL AND METHODS
STUDY AREA
The study was carried out at three different sites of the Divisa River, popularly called "córrego da Divisa", located at the farm São Luís, which is close to the district of Aparecida de Minas belonging to the municipality of Frutal/MG, Brazil, according to its coordinates 20°5'11.09" S, 49°9'19.17" O (Fig. 1).
Sites 1 (P1 - 20° 5' 6.58" S, 49° 9' 21.12" O) and 2 (P2 - 20° 5' 7.25" S, 49° 9' 21.54" O) are characterized as lotic environments, with variations of both its hydric intensity and water flux, having a significant contribution of allochthonous material. Its surrounding area is characterized as a footpath area with riparian vegetation. Differently, site 3 (P3 - 20° 5' 47.97" S, 49° 9' 47.66" O) was an open area, with little vegetation in its surroundings, and a marked prevalence of pastures (bovines and goats) and sugarcane crops. An extensive pig production system exists on the farm, of which the generated effluents were discharged without any previous treatment through piping, directly into the Divisa River.
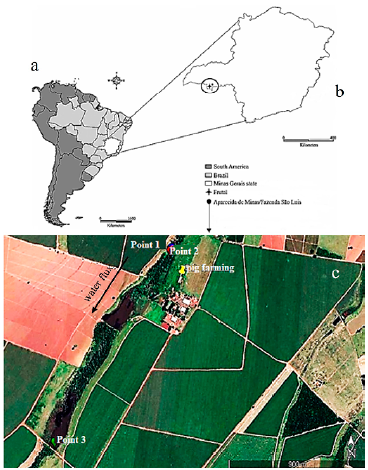
Figure 1 Study area and sampling sites. a) South America/ Brazil; b) Minas Gerais State; c) São Luís Farm. Source: Modified from Fernandes et al. (2015) and Google Maps
The study area presents subtropical climate conditions (Cwa of Koeppen), with dry and rainy seasons and mean temperatures varying between 18.2 and 31.7 °C, with a mean annual temperature of 25.2 °C (Novais et al., 2018). The municipality is part of the Baixo Rio Grande River Basin, with a maximum altitude of 708 meters, a mean altitude of 516 and lower 390 meters (Tomazette et al., 2017). The natural vegetation found in the basin corresponds to the phytogeographic domain of the Cerrado, presenting grassland, "campo-cerrado" (open savanna), cerrado stricto sensu, "cerradão" (savanna), veredas and gallery forest phytophysiognomy (Pereira et al., 2017).
SAMPLE COLLECTION AND LABORATORY ANALYSIS
We performed samplings monthly, between June and November 2018, at the sampling sites previously described, collecting the following limnological variables: temperature, dissolved oxygen (DO), pH, total soluble solids (TSS) and electrical conductivity (EC), measured with the aid of a multi-parameter probe (Horiba U-55).
On the subsurface of the coastal zone, we sampled phytoplankton assemblage using 500 mL polyethylene bottles with three pseudo-replications and acetic lugol 1 % for fixation, and also collected water samples with the aim of quantifying the concentration of total phosphorus (TP), nitrate (NO3), nitrite (NO2) and total ammonium nitrogen (TAN), according to the methods proposed by Koroleff (1976) and Golterman et al. (1978) and quantified with the aid of a spectrophotometer.
We performed a quantitative analysis of phytoplankton in an inverted microscope (Leica DM IL LED), using forty times lenses and ten times eyepiece, and the identification was made up to genus, being grouped in classes using the taxonomic identification keys available in the literature, such as Round (1965, 1971) for Chlorophyceae, Chrysophyceae and Euglenophyceae; Anagnostidis and Komarék (1988, 1990), Komárek and Anagnostidis (1986, 2005), Sant'Anna et al. (2012) for Cyanophyceae and Bicudo and Menezes (2017) for the other observed classes, together with the database of the website AlgaeBase.
We estimated phytoplankton density according to the method described by Utermöhl (1958), using a 10 mL sedimentation chamber. The registers of the principal morphological describers of phytoplankton (cells or colonies) were counted in transects, according to Uehlinger (1964), aiming to quantify at least a hundred organisms of the most abundant species (Lund et al., 1958).
DATA ANALYSIS
To perform an exploratory evaluation of the related variables in each sampling site according to the existing correlations among them (Legendre and Legendre, 2012), we submitted limnological data to a Principal Components Analysis (PCA). To seek statistical differences among sampled sites for each chemical parameter evaluated, we performed a Kruskal-Wallis (H) analysis, considering a 5 % significant level. For this test, only the most representative limnological variables were considered (temperature, TP, NO3, NO2, TAN, TSS, DO and pH).
We tabulated the relative frequency of the phytoplankton genera, to allow the identification of the most frequent genera (constants > 66 %) and perform both the PERMANOVA/SIMPER and CCA analysis based singularly on these genera, which were most representative among the evaluated classes. To verify the differences in phytoplankton composition among sampling spots, we applied the PERMANOVA (Anderson, 2001) based on a Bray-Curtis similarity matrix, followed by the SIMPER analysis based on the Bray-Curtis distance, to demonstrate the which genera contributed most for the dissimilarity among sampled spots.
With the aim of evaluating how phytoplankton classes behave according to the dynamics of limnological variables and sampled sites, we carried out a Canonical Correspondence Analysis (CCA) (Legendre and Legendre, 2012). All statistical analyses were performed using the software Past 2.1 (Hammer et al., 2011), and Excel for the descriptive analysis.
RESULTS
Limnological characterization
The mean water temperature was 23 °C, with the lowest value found in P1 (18.5 °C) and the highest in P3 (26.3 °C). EC varied from 48 (P1) to 75 (P3) μS cm-1, whilst DO have a mean concentration of 4 mg L-1 in P1 and P2 and 5 mg L-1 in P3. The concentration of nitrogen compounds (NO2, NO3 and TAN) displayed a higher variation along with sampling spots, with low concentrations in P1, and higher concentrations in P2, which were gradually reduced in P3. pH values ranged from 5.2 to 7.1 with a tendency to acidity. Regarding TP, P3 showed the highest concentrations in comparison to P1 and P2 (mean 402 μg L-1), being the only limnological variable that was statistically different (p = 0.008) in comparison to the other sites, according to the Kruskal-Wallis' test (Table 1). The concentration of TSS varied from 45 mg L-1 in P3 to 62 mg L-1 in P1. The limnological variables observed in the sampling sites P1, P2 and P3 at the Divisa River are presented in Table 1.
The PCA analysis revealed that the variables that most influenced the first principal component (PC1, 87.27 % of the data variance) were TP, TAN, DO, TSS, pH and NO3 contents, with eigenvalues of 0.98, 0.98, 0.97, 0.97, -0.97 and 0.95, respectively. The second principal component (PC2, 12.73 % of data variance) was influenced by temperature, NO2 and EC, with eigenvalues of -0.72, 0.42 and 0.41, respectively. Both PC1 and PC2 represented together 99.9 % of the data variance (Fig. 2).
Phytoplankton assemblage
The taxa were determined down to genus level and grouped in their corresponding classes, with the most abundant ones of Chlorophyceae (fifteen genus), Cyanophyceae (thirteen genus), Zygnematophyceae (twelve genus), and Bacillariophyceae (ten genus). We found a total of seventy-four genus, distributed in fourteen classes. The classes Chlorophyceae and Cyanophyceae were the ones that mostly contributed to the results in relation to richness, especially in P3, with twelve and ten genera, respectively. The classes that contributed the least were Chrysophyceae, Mediophyceae, Ulvophyceae and Klebsormidiophyceae, which had one genus each.
Among these classes, the ones that presented high contribution in relation to algae density (individuals L-1) were Cryptophyceae (15.000 ind.L-1), Cyanophyceae (13.600 ind.L-1) and Euglenophyceae (8.800 ind.L-1) (Fig. 3). However, by means of the SIMPER analysis that assessed which species most contributed to the dissimilarity among sampling sites, we observed that in P1 and P2, the genus that mostly contributed was Trachelomonas sp., whilst in P3 it was Cryptomonas sp..
Effects of pig breeding treatments on phytoplankton composition
Through the PCA, it was possible to perform an exploratory evaluation of the data and remove certain limnological variables that little explained the variation of other principal components, which were EC and temperature (Fig. 2), and then, the relative frequency of the phytoplankton assemblage was calculated after removing the genera with low occurrence/frequency, such as the ones that were grouped in the following classes: Xanthophyceae, Klebsormidiophyceae, Ulvophyceae, Synurophyceae, and Chrysophyceae. This exclusion of classes was made to perform the analyses PERMANOVA, SIMPER and CCA.
Table 1 Means and standard deviation of the acquired limnological variables on the three sampling sites, and results of the Kruskal-Wallis test, comparing the limnological variables among sampled spots.
| Limnological variables | Mean and Standard Deviation | Test of Kruskal-Wallis (p) | ||
|---|---|---|---|---|
| P1 | P2 | P3 | ||
| E. Conductivity (μS cm-1) (EC) | 75,0 ± 52,0 | 50,0 ± 21,7 | 48,0 ± 22,8 | 0,4 |
| Dissolved Oxygen (mg L-1) (DO) | 4,0 ± 2,4 | 4,3 ± 2,6 | 5,1 ± 3,0 | 0,6 |
| Total Ammoniacal Nitrogen (μg L-1) (TAN) | 12,1 ± 13,1 | 240,7 ± 302,3 | 70,0 ± 73,2 | 0,1 |
| Nitrite (μg L-1) (NO2) | 14,8 ± 15,6 | 40,0 ± 78,7 | 10,9± 11,2 | 0,1 |
| Nitrate (μg L-1) (NO3) | 18,6 ± 27,2 | 35,0 ± 41,0 | 21,0 ± 26,0 | 0,8 |
| pH | 6,4 ± 0,5 | 6,3 ± 0,6 | 6,1 ± 0,7 | 0,7 |
| Temperature (°C) | 22,9 ± 3,0 | 22,6 ± 3,1 | 23,0 ± 3,0 | 0,1 |
| Total Phosphorus (μg L-1) (TP) | 296,3 ± 17,8 | 296,7 ± 59,5 | 402,4 ± 74,7 | 0,008* |
| Total Soluble Solids (mg L-1) (TSS) | 63,0 ± 32,0 | 47 ± 25,5 | 45,0 ± 26,2 | 0,5 |
Caption: * significant level (p < 0.05)
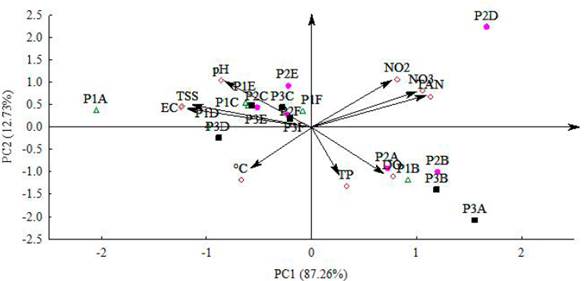
Figure 2- Biplot of the exploratory Principal Component Analysis (PCA) of the limnological variables data set. EC: electrical conductivity; TSS: total soluble solids; pH: hydrogen-ionic potential; °C: water temperature in Celsius degrees; NO2: nitrite; NO3: nitrate; TAN: total ammonium nitrogen; DO: dissolved oxygen; TP: total phosphorus. Sampling sites: P1, P2 and P3. Letters A, B, C, D, E, and F represent the replicates of the sampled spots.
The genus composition did not significantly influence sampling sites, considering a significance level of5 % (PERMANOVA test: total sum of squares = 4.207, within-group squares = 3.48, F = 1.565, p = 0.070). The sites P1 and P2 did not differ from each other (p = 0.979). Furthermore, the sites P1 and P3 (p = 0.04), P2 and P3 (p = 0.048) displayed significant differences among each other.
The SIMPER analysis revealed that the classes Cryptophyceae and Cyanophyceae contributed with 62.75 % for the cumulative dissimilarity between sites P1 and P3, whilst the genera Cryptomonas sp. and Aphanocapsa sp. were the most representative with 24.23 % and 14.29 %, respectively. Between spots P2 and P3, the two genera that have mostly contributed to dissimilarity (64.23 % of the cumulative dissimilarity) were the same, with 24.11% Cryptomonas sp. and 40.12 % Aphanocapsa sp.
Influence of limnological variables on phytoplankton composition
Among all limnological variables initially included in the CCA, the results are usually improved when the direct selection included only seven variables (TSS, NO2, NO3, TAN, pH, DO and TP). The CCA type two grouped phytoplankton classes that were close to the center of axes one and two. Three distinct groups were formed within the gradient, by associating biotic and abiotic variables. The first two ordination axes explained 78.24 % (axis 1: 53.85 % and axis 2: 24.39 %) of the relation between phytoplankton class and limnological variables (eigenvalues of axis 1 = 0.18; and axis 2 = 0.08) (Fig. 4).
A spatial variation of the gradient was observed in P1, dispersing both the biotic and abiotic variables more comprehensively. It was observed that within spots P1A, P2D, and P3D, the class Zygnematophyceae (Zygn) was negatively correlated with NO2, TAN, pH, and TSS. Sites P1 and P2 presented similarities in the distribution between limnological variables and phytoplankton classes. It was also observed that Euglenophyceae (Eugl) and Trebouxiophyceae (Treb) were grouped in spots P1 and P2 (E and F), whilst in P3F it was positively correlated with increased levels of NO3. The classes Dinophyceae (Dino), Cyanophyceae (Cyan), Bacillariophyceae (Baci) and Chlorophyceae (Chlo) were grouped in spots P1 (B, C and D), P2 (A, B and C), and P3 (A, B, C and E), and were positively correlated with NO3, whilst being negatively correlated with TP and DO.
DISCUSSION
The results obtained in this study have showed that pig farming effluents exerted influences in the composition and dynamics of the phytoplankton assemblage, and limnological variables of the Divisa River, presenting high densities of distinct microalgae, such as Cryptomonas sp., Aphanocapsa sp., and Trachelomonas sp., which are organisms capable of inhabiting nutrient-rich environments (e.g., phosphorus and nitrogen in abundance) with high availability of organic matter.
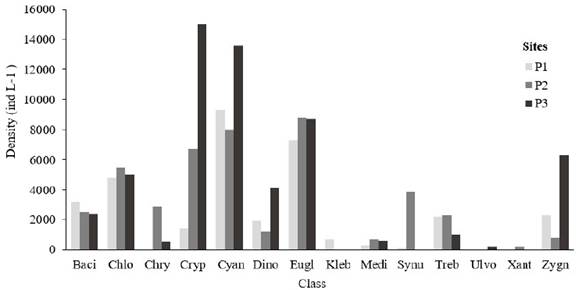
Figure 3- Total density of phytoplankton classes sampled from June to November 2018 at the Divisa River - Aparecida de Minas/MG. Caption: Baci: Bacillariophyceae; Chlo: Chlorophyceae; Chry: Chrysophyceae; Cryp: Cryptophyceae; Cyano: Cyanophyceae; Dino: Dinophyceae; Eugl: Euglenophyceae; Kleb: Klebsormidiophyceae; Medi: Mediophyceae; Synu: Synurophyceae; Treb: Trebouxiophyceae; Ulvo: Ulvophyceae; Xant: Xanthophyceae; Zygn: Zygnematophyceae. Sampling sites: P1, P2 and P3.
High concentrations of TP were found, especially in P3, where large amounts of floating macrophytes of the genus Eichhornia. Among the central pollutants of pig farming effluents are phosphorus and nitrogen, which are known as the most limiting macronutrients for algae growth in continental ecosystems, thus being one of the drivers of eutrophication (Palhares and Calijuri, 2007, Vieira et al., 2009). In addition, P3 was the spot that registered that highest number of individuals belonging to classes Chlorophyceae and Zygnematophyceae, as well as the highest densities, including Cryptophyceae, Cyanophyceae and Euglenophyceae, which were different in comparison to phytoplankton composition of P1 and P2.
The presence of a macrophyte bank in P3 possibly helped in a positive way, absorbing compounds such as phosphorus and nitrogen in high concentrations, and increasing the oxygen concentration (Esteves, 2011). On the other hand, Bucci and Oliveira (2014) highlighted that the proliferation of aquatic macrophytes is related to high concentrations of nutrients, such as phosphorus and nitrogen, and to anthropic interferences that begin to emerge from the damming process itself. Thus, such a phytoremediation capacity in retaining/filtrating organic materials from a specific site to upstream locations will not always be effective and might cause an acceleration of the eutrophication process (Klein and Agne, 2012).
In P2, we found high concentrations of NO2, but NO3, DO and the temperature was low. Such a high concentration of nitrogen compounds is possibly an indication of the disposal of effluents without prior treatment or even an influence on the river surrounding environment. The phytoplankton composition in P2 presented a high density of Euglenophyceae and Cyanophyceae individuals, which are considered cosmopolitan algae, being found in mesotrophic and eutrophic environments (Castro and Moser, 2012).
Ammonium is the form preferentially assimilated by phytoplankton (Miwa et al., 2007), which in high concentrations may cause major ecological implications, by strongly influencing the dynamics of DO and pH, corroborating the studies of Batista et al. (2017), and increasing primary phytoplankton productivity (Cardoso Silva et al., 2014). As shown by the CCA, spots P2B, P2C and P2D had Cyanophyceae, Bacillariophyceae and Chlorophyceae, which were positively correlated with NO2, DO and TP and corroborate the results presented by Aprile and Mera (2007).
The variables EC, TSS and NO3 were high in P1, unlike TP and TAN, which were low on this site. High concentrations of suspended solids inhibit the penetration of light in the water column, so that it interferes the photosynthesis performed by aquatic organisms (Herawati et al., 2019). According to Von Rückert and Giani (2004), NO3 is not toxic for aquatic organisms, but when its concentration is excessively high, it may lead to excessive growth of microalgae, which in turn might explain the high density and richness of the filamentous Cyanophyceae found in this spot.
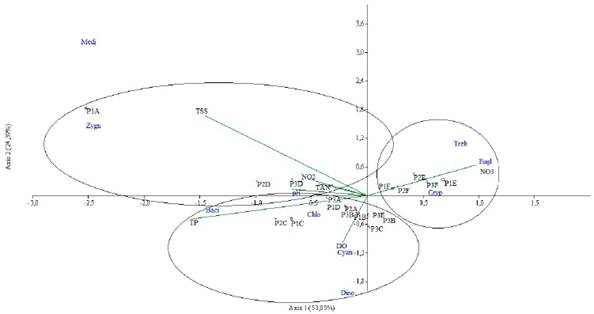
Figure 4- Results of the CCA of species composition, using all explicative variables, which include TSS: total soluble solids; pH: hydrogen-ionic potential; NO2: nitrite; NO3: nitrate; TAN: total ammonium nitrogen; DO: dissolved oxygen; TP: total phosphorus. The most representative classes were Baci: Bacillariophyceae; Chlo: Chlorophyceae; Cryptophyceae; Cyano: Cyanophyceae; Dino: Dinophyceae; Eugl: Euglenophyceae; Medi: Mediophyceae; Treb: Trebouxiophyceae; Zygn: Zygnematophyceae. Sampling spots: P1, P2 and P3. Letters A, B, C, D, E, and F represent the replicates of the sampled sites.
Using the PERMANOVA and SIMPER analyses, it was possible to observe the phytoplankton classes that most contributed for the dissimilarity among sampling sites, being: Cryptophyceae, Cyanophyceae and Euglenophyceae, represented by the genera Cryptomonas, Aphanocapsa and Trachelomonas, respectively. Nevertheless, Cryptophyceae has contributed to all sampled sites, and these microalgae are frequently found in shallow environments with low light intensity and high nutrient concentration, with the presence of currents and submerged macrophytes (Moura et al., 2013). Other studies have also observed the great contribution of Cryptophyceae algae in both lotic and lentic environments (Reynolds et al., 2002; Strandberg et al., 2015; Abirhire et al., 2016; Aquino et al., 2018).
CONCLUSION
We concluded that increased concentration of nutrients, such as phosphorus and nitrogen compounds, have influenced the occurrence of a few groups of phytoplanktonic microalgae (Cyanophyceae, Cryptophyceae and Euglenophyceae), which are commonly found in shallow, low-light environments, with high concentrations of organic matter, being tolerant to water currents. Therefore, further studies considering phytoplankton should be developed in Brazilian lotic environments, to improve knowledge about the biological diversity and energetic balance in different habitats and to contribute to the conservation of aquatic ecosystems.

